Gregor Johann Mendel: Father of Genetics Explained
By Dr. Zubair Khalid, DVM, MS, PhD ·
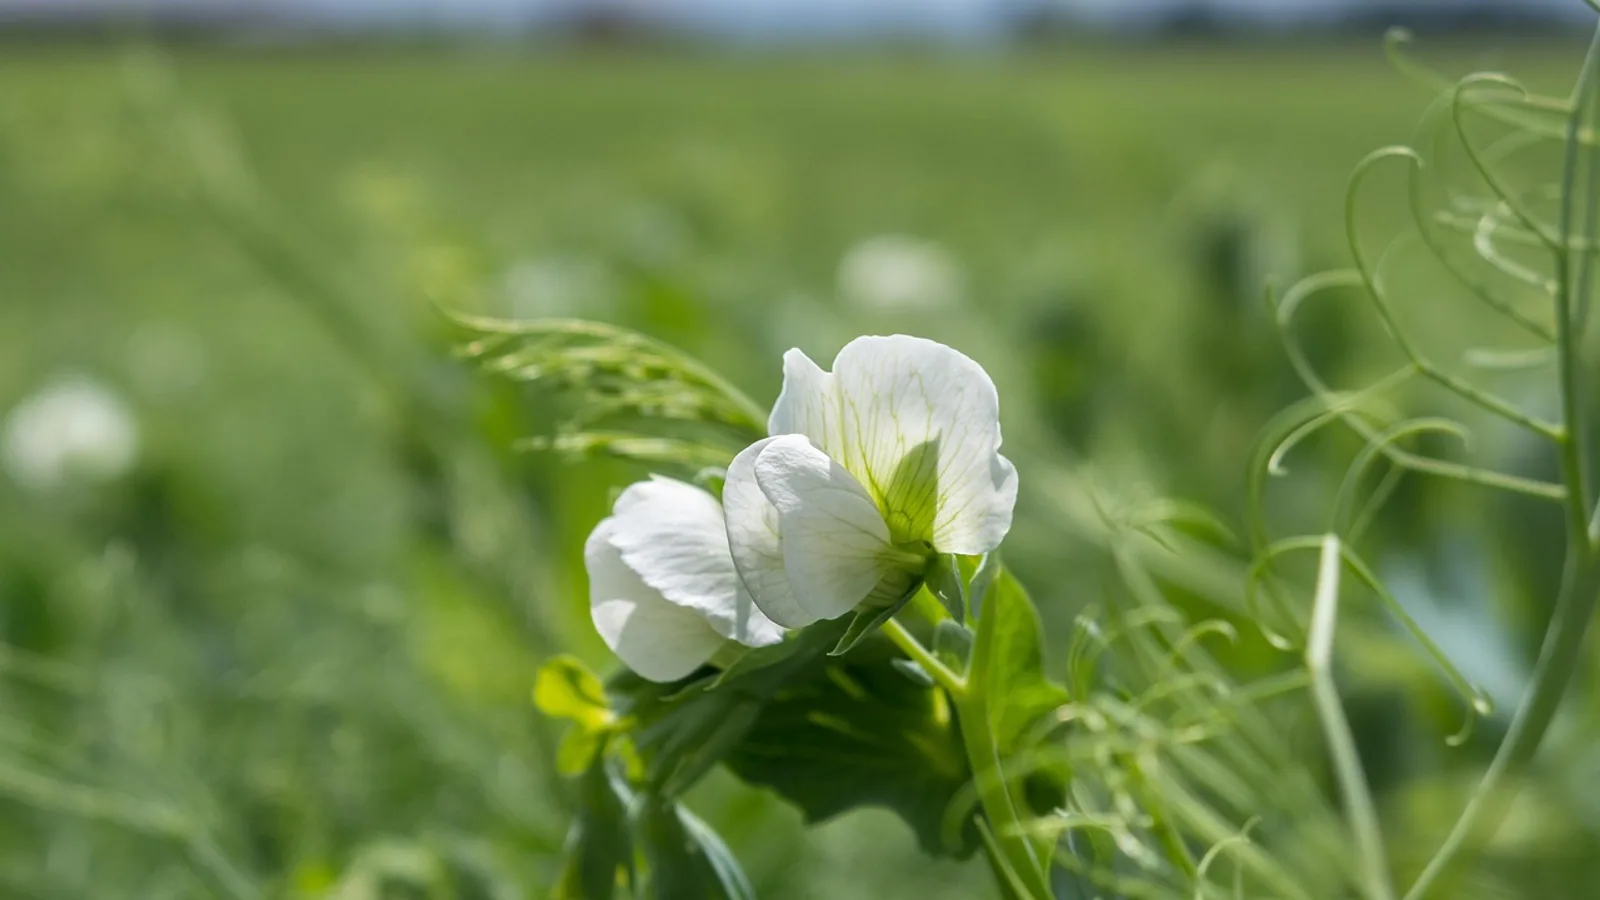
Gregor Johann Mendel was an Augustinian friar and plant breeder in Brno who, between 1856 and 1863, crossed thousands of pea plants and counted their offspring trait by trait. From those counts he derived the first quantitative laws of inheritance, presented publicly in 1865 and published in 1866, which is why he is called the father of genetics.
Who Was Gregor Johann Mendel?
Mendel was born on July 20, 1822, in Heinzendorf, a village in the Kuhländchen, a predominantly German-speaking area of northern Moravia, then part of the Austrian Empire [1]. He was born into a humble farm family. His academic gifts were clear early, but his father's accident and subsequent incapacity left the family unable to fund his higher studies, and the resulting financial strain and illness threatened his ability to finish his education at all [1].
The path he found was the Augustinian monastery of St. Thomas in Altbrünn, now Staré Brno, a district of Brno. There he completed theological studies and was ordained. Practical pastoral work did not suit him. He was psychosomatically unsuited to parish duties and was instead directed toward teaching, though he lacked the state certification required for a permanent post, and an attempt to pass the certification examination failed [1].
That failure turned out to be the most consequential event in the history of genetics. The monastery sent him to the University of Vienna for a two-year course of study with emphasis on physics and botany, partly to prepare him for a second attempt at the exam [1]. The training he received there in experimental physics and in botanical method gave him the tools he later applied to heredity. He learned to design controlled experiments, to count, and to reason about ratios. Those are not the instincts of a naturalist collecting specimens. They are the instincts of a physicist, and they shaped everything that followed.
Mendel died on January 6, 1884, in Brno. His work was largely set aside by the scientists of his day and was rediscovered around 1900, independently, by Hugo de Vries, Carl Correns, and Erich von Tschermak.
What Was Mendel Actually Trying to Do?
The standard telling of the Mendel story often implies that he set out from the beginning to discover the laws of heredity. The historical record is more interesting. Two local newspaper articles about Mendel's work, published four years before his famous Pisum lectures, describe him as a plant breeder and horticulturist [2]. The picture that emerges is that his initial interests concerned crop improvement, and that only over time did he become more interested in fundamental questions about inheritance, fertilization, and natural hybridization [2].
This matters for how his experiments are read. Mendel was working in a tradition. The Moravian Agricultural and Natural Science Society in Brno was a serious scientific body whose members debated the improvement of sheep wool for the Habsburg armies, and who argued about how "climate" or "seed" characteristics influenced wool quality and quantity [3]. Breeders and academics in that circle put their knowledge into immediate practice, creating animals with better wool traits through consanguineous matching and artificial selection [3]. Mendel was embedded in a culture that thought hard about heredity because heredity had economic consequences.
He was also not the only person thinking about these problems. The history of heredity before Mendel is a long one, and the standard textbook sketch that jumps from nothing to Mendel does students a disservice [4]. Understanding what his contemporaries debated helps explain why he asked the questions he did and why he planned his pea studies the way he did [4].
Why Peas?
Mendel chose the garden pea, Pisum sativum, deliberately, and the choice was excellent. Peas have several properties that make them ideal for inheritance studies.
First, peas are naturally self-pollinating, which means a plant normally fertilizes itself. This gives the researcher stable, true-breeding lines. Second, the flowers are large enough that a researcher can open a bud, remove the anthers before they shed pollen, and apply pollen from another plant by hand. This gives complete control over which plant fertilizes which. Third, peas produce many offspring per cross, which matters enormously when you are trying to detect a 3:1 ratio. Fourth, peas have discrete, unambiguous traits. A seed is either round or wrinkled. A flower is either purple or white. There is no subjective judgment in scoring.
Mendel studied seven pairs of contrasting traits in pea in detail, and these seven pairs established the foundational principles of genetic inheritance [5]. They are:
- Seed shape: round versus wrinkled
- Seed color: yellow versus green
- Flower color: purple versus white
- Flower position: axial (along the stem) versus terminal (at the top)
- Pod shape: inflated versus constricted
- Pod color: green versus yellow
- Stem length: tall versus short
Modern genomics has now identified the genes and alleles behind all seven. Researchers have uncovered previously undescribed alleles for the four characterized Mendelian genes, including a rare revertant of Mendel's white-flowered a allele [5]. For the three remaining traits, the picture is now clear. An approximately 100-kb genomic deletion upstream of the chlorophyll synthase gene (ChlG) disrupts chlorophyll biosynthesis through the generation of intergenic transcriptional fusion products, conferring the yellow pod phenotype [5]. A MYB gene with an upstream Ogre element insertion and a CLE peptide-encoding gene with an in-frame premature stop codon explain the v and p alleles, which disrupt secondary cell wall thickening and lignification, producing the parchmentless, edible-pod phenotype [5]. A 5-bp exonic deletion in a CIK-like co-receptor kinase gene, combined with a genetic modifier locus, is associated with the fasciated stem phenotype [5].
That is a remarkable outcome. A friar counting peas in the 1850s identified seven traits whose molecular basis we can now specify to the base pair.
Mendel's Method
Mendel's experimental design was the key to his success. He began by establishing true-breeding lines for each trait. He then performed crosses between lines that differed in one trait (monohybrid crosses) and later between lines that differed in two traits (dihybrid crosses).
He also did the reciprocal cross. He pollinated a round-seeded plant with pollen from a wrinkled-seeded plant, and he did the reverse. The results were the same either way, which told him that both parents contribute equally to the offspring.
He then allowed the first-generation hybrids to self-pollinate and counted the second generation. This is the step that most people before him had skipped. Many breeders had noticed that hybrids sometimes resembled one parent and sometimes the other, but nobody had systematically counted the offspring of hybrids across many generations and many traits.
Mendel also introduced a vocabulary that we still use. He introduced the terms "dominant" and "recessive" characters and determined their 3:1 ratio in the offspring of heterozygous hybrid plants [6]. A dominant character is the one that appears in the hybrid. A recessive character is the one that disappears in the hybrid and reappears in the next generation.
The Law of Segregation and the 3:1 Ratio
The monohybrid cross is the core of Mendelian genetics. Consider seed shape. Mendel crossed a true-breeding round-seeded plant with a true-breeding wrinkled-seeded plant.
The first filial generation, or F1, was entirely round. Every single plant. The wrinkled trait had vanished.
Mendel then let the F1 plants self-pollinate. In the second filial generation, or F2, both traits reappeared. Round and wrinkled. When he counted, the ratio was approximately 3 round to 1 wrinkled.
The explanation is that each plant carries two copies of a hereditary factor, one from each parent. Mendel called these factors "elements." We now call them alleles, which are alternative versions of a gene. The true-breeding round parent carries two copies of the round allele. The true-breeding wrinkled parent carries two copies of the wrinkled allele. The F1 plant carries one of each, and because round is dominant, the F1 plant looks round.
When the F1 plant makes gametes, the two alleles separate. Each gamete gets one or the other, with equal probability. This is the Law of Segregation. When two F1 plants are crossed, four combinations are possible in the offspring, and three of them contain at least one round allele.
A Worked Monohybrid Punnett Square
Let us assign symbols. Let R be the dominant round allele and r be the recessive wrinkled allele. The true-breeding round parent is RR. The true-breeding wrinkled parent is rr. The F1 plant is Rr.
To predict the F2 generation, we write the possible gametes from each F1 parent along the two axes of a Punnett square. Each F1 parent produces R gametes and r gametes in equal numbers.
| R (from parent 1) | r (from parent 1) | |
|---|---|---|
| R (from parent 2) | RR | Rr |
| r (from parent 2) | Rr | rr |
Reading the four boxes:
- RR: one box out of four, or 1/4. Homozygous dominant. Round seed.
- Rr: two boxes out of four, or 2/4. Heterozygous. Round seed, because R is dominant.
- rr: one box out of four, or 1/4. Homozygous recessive. Wrinkled seed.
The genotypic ratio is 1 RR : 2 Rr : 1 rr. The phenotypic ratio is 3 round : 1 wrinkled. That is the 3:1 ratio Mendel observed, and it falls directly out of the mechanics of segregation.
Note the terminology. A homozygote carries two identical alleles at a locus. A heterozygote carries two different alleles. The genotype is the allele combination. The phenotype is the observable trait. The terms dominant and recessive describe the relationship between alleles at the level of the phenotype, not the strength or importance of the allele itself.
The Law of Independent Assortment and the 9:3:3:1 Ratio
Mendel then asked whether traits are inherited together or independently. He crossed plants that differed in two traits at once, for example round yellow seeds versus wrinkled green seeds.
The F1 generation was entirely round and yellow. When he allowed the F1 plants to self-pollinate, the F2 generation showed four phenotypic classes in a ratio of approximately 9:3:3:1.
- 9/16 round yellow
- 3/16 round green
- 3/16 wrinkled yellow
- 1/16 wrinkled green
The critical observation is that the combinations that were not present in either parent, round green and wrinkled yellow, appeared in the F2. This told Mendel that the two traits assort independently of one another during gamete formation. This is the Law of Independent Assortment.
The 9:3:3:1 ratio is simply two 3:1 ratios multiplied together. If seed shape gives 3:1 and seed color gives 3:1, then the joint distribution is (3:1) × (3:1), which expands to 9:3:3:1. This is why the dihybrid ratio is not a separate law but a consequence of two monohybrid ratios behaving independently.
What Mendel's "Factors" Are Now Called
Mendel's "factors" or "elements" are now called alleles. The term "gene" came later, and its etymology is a historical curiosity. The word evolved from Darwin's imagined "gemmules," not from Mendel's factors [7]. Darwin proposed a theory of heredity called pangenesis, in which particles called gemmules were shed by all parts of the body and collected in the gametes. That theory was wrong in its mechanism, but the word stuck.
The modern definition is straightforward. A gene is a segment of DNA that encodes a functional product, usually a protein or a functional RNA. A locus is the physical position of a gene on a chromosome. An allele is one of the alternative versions of a gene that can exist at a locus. A diploid organism carries two alleles at each autosomal locus, one inherited from each parent.
Mendel had no knowledge of chromosomes, DNA, or meiosis. He inferred the existence of paired, separable factors purely from the ratios he observed. That inference was correct.
Why Was Mendel's Work Rediscovered Around 1900?
Mendel presented his work publicly in 1865 and published it in 1866 in the proceedings of the Natural History Society of Brno. It was cited a handful of times and then largely forgotten. Around 1900, three botanists working independently, Hugo de Vries, Carl Correns, and Erich von Tschermak, each arrived at similar conclusions and each found Mendel's paper in the literature. The rediscovery launched genetics as a formal science.
The reasons for the earlier neglect are debated and often oversimplified. What is documented is that Mendel himself tried to extend his work beyond pea and ran into trouble. He wrote to Carl von Nägeli, a leading botanist, that he believed he needed to verify, with other plants, the results obtained with Pisum [8]. For this purpose he adopted Hieracium subgenus Pilosella, a phenotypically diverse taxon under botanical study at the time [8].
The choice was disastrous, and not through any fault of Mendel's reasoning. The majority of Hieracium plants are not sexual like pea. They are facultatively apomictic, meaning the majority of seed arises asexually and the progeny are clones of the maternal parent [8]. Mendel obtained very few hybrids in his Hieracium crosses. Researchers have calculated that he probably emasculated in excess of 5,000 Hieracium florets to obtain even the small numbers he did [8]. He was perplexed by the results, and they ultimately led him to conclude that the hybrids of Hieracium show a behavior exactly opposite to those of Pisum [8].
This is a genuine limitation of the pea work as his contemporaries saw it. One apparent criticism was that his findings only applied to pea [8]. Mendel knew this was a vulnerability and tried to address it. He failed, for reasons that had nothing to do with the validity of his laws and everything to do with the reproductive biology of the plant he happened to pick.
Mendel also conducted controlled pollination experiments in Mirabilis jalapa during his later research period. Two letters to Nägeli record that the experimental aim was to disprove Darwin's opinion that three pollen grains were required for one fertilization, an idea that would have destroyed his previous discovery of segregation inheritance in variable hybrids in Pisum [9]. The results of single pollen grain pollination confirmed that one pollen cell unites with one egg cell in plant fertilization, and the pedigree experiments succeeded in showing that one hereditary factor carried by one gamete can independently transmit a trait to offspring [9]. This body of work supports what has been called the gamete theory of inheritance [9].
Linkage and Exceptions Do Not Invalidate Mendel's Laws
Two complications are worth addressing directly, because they are the most common source of confusion for students.
The first is linkage. Mendel's Law of Independent Assortment holds for genes on different chromosomes, or for genes far apart on the same chromosome. Genes that are physically close together on the same chromosome tend to be inherited together, because the chromosome is the unit that segregates during meiosis. Recombination can separate them, but the closer they are, the less often that happens. Linkage was discovered after Mendel's work was rediscovered, and it refines the law rather than refuting it. Independent assortment is the default. Linkage is the exception that has a physical explanation.
The second is the broader category of non-Mendelian inheritance. Mendel's framework describes the behavior of nuclear genes with simple dominant and recessive relationships. Many real genes do not behave that simply. The genetics literature now recognizes incomplete dominance, codominance, pleiotropy, epistasis, imprinting, and many other phenomena [10] [6]. In clinical genetics, the transmission pattern of a disorder may depend not only on the character but also on the genetic background, modifiers, and other factors [6].
Mendel himself was aware of more than the textbook version of his work suggests. His theory is considerably richer than the two principles it is usually reduced to, encompassing the nature of fertilization, the role of hybridization in evolution, and aspects often considered as exceptions or extensions, such as pleiotropy, incomplete dominance, and epistasis [11]. He researched hybridization in at least twenty plant genera and intentionally chose some species whose inheritance he knew would deviate from the patterns he observed in the garden pea [11].
None of this invalidates the laws. Segregation and independent assortment describe what happens to alleles and chromosomes during gamete formation. They are the baseline. Everything else is a modification layered on top of that baseline.
Common Mistakes and Limitations
Treating dominant as meaning "more common." Dominance describes the phenotype of a heterozygote, not the frequency of an allele in a population. A dominant allele can be rare. A recessive allele can be common.
Confusing genotype and phenotype. The genotype is the allele combination. The phenotype is the observable trait. A round pea can be RR or Rr. You cannot tell which from looking at it.
Assuming a 3:1 ratio appears in small families. The 3:1 ratio is a statistical expectation over many offspring. In a family of four, you might see four round peas and no wrinkled ones by chance alone. Mendel succeeded partly because he counted thousands of plants.
Believing Mendel's laws apply to every gene. They apply to nuclear genes that segregate and assort in the standard way. Mitochondrial genes, imprinted genes, and genes subject to meiotic drive do not follow the same rules [10].
Reading the data-reliability debate as a scandal. Mendel's data show a remarkable agreement with his predicted ratios, closer than standard statistical models would predict [12]. Various explanations have been tested, including the possibility that inheritance in pea naturally produces ratios closer to Mendelian expectations, that data were omitted, that ambiguous phenotypes were miscategorized, and that some data were deliberately falsified [12]. The possibility that pea naturally produces segregation ratios more closely matching Mendelian expectations has been rejected, and in fact the opposite was found, making Mendel's results even more remarkable [12]. Considerable evidence indicates that Mendel omitted some experimental results, but this does not adequately explain the low average deviation from expectations in the segregation data he presented [12]. An underlying bias favoring the predicted ratio is present, but the analysis could not clearly determine whether it came from misclassifying ambiguous phenotypes or deliberate falsification [12]. A number of Mendel's statements are argued to be unrealistic in terms of practical pea genetics, suggesting his text does not represent a strictly accurate description of his methods [12]. This is a live scholarly question, not a settled verdict.
Assuming Mendel was ignored because nobody understood him. The documented reasons are more specific. His pea findings were seen as possibly applying only to pea, and his own attempt to extend them to Hieracium failed because that plant reproduces asexually [8].
Individual clinical cases require professional evaluation. Nothing here substitutes for a genetic counselor or physician when a real inheritance question arises.
Practical Implications
Mendel's framework is still the working tool of applied genetics. In plant breeding, the same logic he used to design pea crosses is used to design crosses in every major crop. Legumes in particular have played an important part in cropping systems since the dawn of agriculture, and the pea was the original model organism used in Mendel's discovery of the laws of inheritance, making it the foundation of modern plant genetics [13].
In medicine, Mendelian inheritance remains the first analytical tool for a suspected monogenic disorder. The 3:1 ratio in the offspring of heterozygous carriers allows calculation of the number of phenotype-determining alleles and has been used ever since to prove the monogenic origin of a disorder [6]. The Mendelian inheritance of monogenic kidney disorders, for example, still helps distinguish them from disorders with multifactorial origin in clinical practice [6]. The equal contribution of the two parents, the direct correlation between the frequency of a recessive character and the degree of inbreeding, and complete penetrance in simple cases all follow from Mendel's observations [6].
In evolutionary biology, the rediscovery of Mendel in the early 20th century led to two reforms of Darwinism, Neo-Darwinism and the Modern Synthesis [14]. Darwin's proximate processes of evolution predated the discovery of genetics, and the laws of inheritance filled that gap [14].
Frequently Asked Questions
When was Gregor Johann Mendel born and when did he die?
Mendel was born on July 20, 1822, in Heinzendorf in northern Moravia, and he died on January 6, 1884, in Brno [1].
What were the seven pea traits Mendel studied?
Seed shape (round versus wrinkled), seed color (yellow versus green), flower color (purple versus white), flower position (axial versus terminal), pod shape (inflated versus constricted), pod color (green versus yellow), and stem length (tall versus short) [5].
What is the 3:1 ratio in Mendel's experiments?
It is the ratio of dominant to recessive phenotypes in the second generation of a monohybrid cross, arising because three of the four possible allele combinations in the offspring contain at least one dominant allele [6].
What is the 9:3:3:1 ratio?
It is the ratio of the four phenotypic classes in the second generation of a dihybrid cross, and it is the product of two independent 3:1 ratios.
What did Mendel call the units of inheritance?
He called them factors or elements. We now call them alleles, which are alternative versions of a gene at a given locus.
Who rediscovered Mendel's work and when?
Hugo de Vries, Carl Correns, and Erich von Tschermak independently rediscovered it around 1900, roughly 34 years after Mendel published and 16 years after he died.
Why did Mendel's experiments with Hieracium fail?
Most Hieracium species are facultatively apomictic, meaning they produce seed asexually, so Mendel's crosses produced clones of the maternal parent rather than hybrids [8].
Do linkage and non-Mendelian inheritance disprove Mendel's laws?
No. Linkage and phenomena like incomplete dominance, epistasis, and imprinting are refinements that operate on top of the segregation and independent assortment of alleles [10] [6].
Related Articles
- Is Dog Separation Anxiety Genetic
- How to Read the Genetic Code: A Comprehensive Guide
- A Guide to Genetic Counseling: Principles and Practice
- Genetic Diseases in Animals: Mechanisms and Examples
- Calico Cat: Fascinating Facts and Genetics Explained
- Tortoiseshell Cat: Personality, Health, and Genetics
- Genetic Transduction: How Phages Move Bacterial Genes
- Araucana Hen Eggs: Blue Egg Genetics and Care
Sources
- Historical study: Johann Gregor Mendel 1822-1884.
- How Mendel's Interest in Inheritance Grew out of Plant Improvement.
- Mimush Sheep and the Spectre of Inbreeding: Historical Background for Festetics's Organic and Genetic Laws Four Decades Before Mendel's Experiments in Peas.
- Principles and biological concepts of heredity before Mendel.
- Genomic and genetic insights into Mendel's pea genes.
- The dominant findings of a recessive man: from Mendel's kid pea to kidney.
- Darwin and Mendel today: a comment on "Limits of imagination: the 150th Anniversary of Mendel's Laws, and why Mendel failed to see the importance of his discovery for Darwin's theory of evolution".
- Seeds of doubt: Mendel's choice of Hieracium to study inheritance, a case of right plant, wrong trait.
- Mendel's controlled pollination experiments in Mirabilis jalapa confirmed his discovery of the gamete theory of inheritance in Pisum.
- From Mendel's laws to non-Mendelian inheritance.
- Demystifying the mythical Mendel: a biographical review.
- Are Mendel's Data Reliable? The Perspective of a Pea Geneticist.
- Legume Genetics and Biology: From Mendel's Pea to Legume Genomics.
- From Darwin's Origin of Species toward a theory of natural history.